A major error occurred when scientists decreed that only naturalistic explanations could be used to explain the origin of life and how it operates. Decades of molecular biology research have produced an extraordinary catalogue of cellular details, yet a coherent, unified explanation of how cells function as a whole is lacking.1 Rafelski and Theriot pointed out that2
“The living nature of the cell inherently means that we cannot make the same simplifying assumptions that we typically use for many other complex dynamical systems, and we cannot assume that we fully understand the nature of the laws that govern cell behavior.”
The naturalistic scientific community insists that only purely material, undirected chemical processes must account for the emergence of life. However, this focus on chemical reactions has sidetracked from the fundamental biological questions that needed to be answered. Cells are the foundation of life, and it is precisely their defining properties that require an explanation. They must autonomously grow, adapt, self-protect, self-repair, recycle components, manufacture their own hardware, and reproduce with astonishing fidelity across countless generations.
No collection of abiotic chemical reactions has ever been observed to bootstrap itself into this kind of integrated, purposeful system. More than 99% of reactions relevant to biological systems are catalyzed by tailor-designed genetically encoded protein catalysts. EcoCyc version 24.5 records 1,682 curated metabolic enzymes (those directly catalyzing small-molecule transformations) for the model bacterium E. coli K-12, plus 288 transporters catalyzing transport reactions. In addition, there are many nucleases, proteases, kinases, and other classes of enzyme. Without these enzymes the reactions would be too slow and inefficient. Details like these should have shown the disconnect between prebiotic chemical research and living systems.
Truman et al. addressed this misdirection by proposing a top-down computational paradigm: cells are best understood as integrated multiprocessing analogue computing devices. Daughter cells inherit cryptic computational logic that directs biochemical processes, anticipating future requirements with flexible responses.
Cellular design interpreted as analogue computing
Unlike digital computers, pure analogue processors do not require software code separate from the hardware; the physical construction is the programme. The implications for cells are profound. Cells operate through thousands of molecular Recognition Elements (REs) that can be viewed as sensors, which respond to continuous gradients of Specificity Factors (SPs), which are sometimes called ‘signals’. These REs function as programming variables—dynamic biological elements capable of initiating and regulating cascades of downstream processes. The outcomes depend on the magnitude, duration, and context of the SPs they detect. Truman et al. documented many examples of this principle, with SP effectors ranging from transcription factors and glucose to calcium ions and mechanical strain, each producing graded, continuous regulatory outputs. This analogue character is pervasive: it is observed in signal transduction pathways, metabolic feedback inhibition, cell cycle control, chromatin dynamics, developmental gradients, immune responses, etc.
Furthermore, the responsiveness of REs can be modified. Ligand attachments, chemical modifications (phosphorylation, methylation, glycosylation), cofactors, pH, and temperature all fine-tune the response to the same concentration gradient. This represents a qualitatively richer form of programming than anything available in digital systems.
The logic of cellular programming
Identifying cellular REs as programming variables is a key conceptual advance of this framework. In digital computing, variables are abstract locations in memory where values are stored and retrieved. In cells, REs are physically positioned at specific molecular locations—on DNA, RNA, proteins, lipids, and carbohydrates—where they respond to SPs. The logical operations are directly implemented physically: SP binding to RE constitutes the assignment of a value, and this assignment initiates downstream processing.
This relationship has properties that transcend ordinary chemical interaction. Cellular variables must be unambiguous, are used to communicate intention, can perform operations, and may recursively represent collections of other variables.
A further key insight is the distinction between the immediate goal and the major goal of a cellular variable. The immediate goal is the physical recognition event: a codon identifying the correct anticodon; a receptor, tyrosine kinase, recognizing its extracellular ligand; or a TATA-binding protein recognizing its eight-nucleotide promoter sequence. This physical recognition event is only the initiating step—Step 1. The major goal—Step 2—is the downstream functional outcome: protein synthesis, gene activation, chromatin remodelling, signal transduction cascade, etc. The entire downstream machinery is assembled in response to the RE–SP interaction. This just-in-time assembly and disassembly of processing hardware ensures efficient use of cellular resources.
Adaptor molecules and if–then logic
Cellular decision-making is implemented through a recursive, cascading logic in which each RE–SP interaction generates a new microenvironment that serves as a new RE for the next step. This is exemplified by adaptor molecules. The tRNA is a canonical single-adaptor molecule: one end identifies a specific mRNA codon while the other end carries the correct amino acid.
More commonly, cells implement logic through multi-component adaptor complexes, in which each recruited protein or RNA possesses both an RE for its upstream partner and an RE for the next component in the assembly chain. The concept of adaptor molecules and complexes is shown in figure 1. This recursive, stepwise logic describes many key cellular processes.
The power of the framework was demonstrated through many examples of REs, placed on DNA, RNA, and proteins. In every case, the RE possesses a distinctive recognition feature embedded within a supporting molecular housing, which optimizes binding, excludes false binding partners, and ensures the interaction is coupled to a specific downstream process. The engineering required to regulate a multitude of processes concurrently—in the same cellular volume, and without catastrophic interferences—is far beyond current human technologies.
Advantages of analogue design in cells
Four advantages of using analogue technologies in cells include:
- Analogue regulation permits fine-tuned, graded responses, which avoid waste and optimize resource allocation.
- Responding directly to concentration-gradients is simpler than discretizing gradients into discrete intervals and computing separate logic for each interval.
- Analogue binding interactions—relying on multiple small non-covalent contributions (hydrogen bonds, van der Waals forces, hydrophobic interactions, ionic bonds)— confer robustness to individual mutations. No single point change abruptly abolishes function; the system degrades gracefully.
- The use of thousands of dedicated, simple, modular molecular machines—assembled just in time and dismantled when no longer needed—is far superior to a monolithic general-purpose processor. For example, up to 10 million ribosomes operate concurrently in human liver cells, while red blood cells have none; up to 100,000–200,000 spliceosomes are active in many cell types concurrently. The copy number of each machine can be regulated dynamically according to cell type, stage in the cell cycle, and immediate cellular needs. This modularity enables rapid scaling, precise replacement of defective components, and efficient recycling of molecular raw materials.
Implications for origins: design, not chemistry
The cumulative force of this framework carries direct implications for the origins debate. A cell is not merely a complex chemical system; it is an integrated, multiprocessing, self-manufacturing, self-repairing, self-reproducing collection of analogue computing devices (fig. 2).
Chemical systems, however complex, do not produce REs that encode intended outcomes unrelated to their own physical binding properties. They do not assemble just-in-time machinery. They do not regulate copy numbers of their own processing hardware. They do not implement recursive if–then logic across thousands of concurrent programmes. They do not pass all of this in a fully operational state to daughter systems, generation after generation.
The gulf between regulated cellular biochemistry and abiotic chemical processes is qualitative, not merely quantitative. No incremental sequence of undirected chemical steps bridges this gulf, because the gulf is not one of chemical complexity but of information architecture—the very thing that origin-of-life models are least equipped to explain.
The research programme initiated by Truman et al. points towards the concept of analogue metaprogramming in cells: the phenomenon whereby parametrized cryptic encoded information unfolds to generate complex programs. This intuition has been proposed by computer science professor Uwe Assmann during several creation science workshops in Germany and will be communicated in later papers. This recursive generativity—hardware that builds hardware—is a hallmark of sophisticated, intentional engineering. It is the kind of feature that, if found in an extra-terrestrial location, would unhesitatingly be attributed to an intelligent designer.
REs are used by all biological codes and usually in vast copy numbers. This enables massive parallel processing. A well-known example is DNA replication in mammals, that relies on tens of thousands of replication origins, so that billions of base pairs can be copied in parallel sections. In a paper in this edition, I argue that the probability of correctly positioning enormous numbers of REs through random mutation and selection is prohibitively low. The paper further points out that evolving new biological codes would require large amounts of additional non-functional genetic material, which population genetics predicts would impose selective disadvantages that make fixation in populations prohibitively unlikely.
Conclusion
The analogue computing framework presented by Truman et al. offers what no chemistry-first model has provided: a coherent, top-down, systems-level account of how cells actually function. Thousands of sensors, implemented across DNA, RNA, proteins, and other biomolecules, respond to continuous signal gradients and initiate cascading, purposeful, recursive programmes. Hardware and software are inseparably integrated. Molecular machinery is manufactured, deployed, and recycled on demand. The entire system reproduces itself faithfully across generations, the result of a top-down design set in motion with each class of original cell. Importantly, complex processes like cell cycle, morphogenesis, immunity, and neurobiology require coordinated regulation of multiple subprocesses,15 all relying on analogue coding programmes.
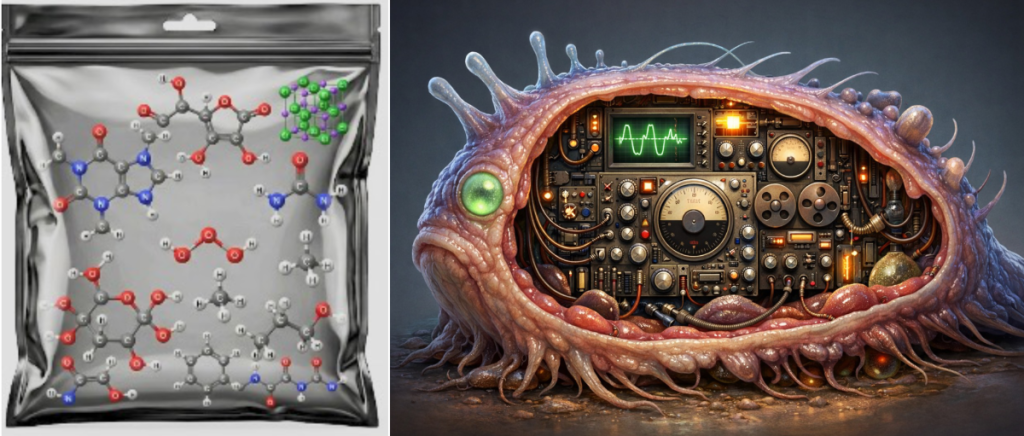
This image contrasts the view of cells as a collection of chemical reactions vs a sophisticated information-processing technology. Cells are not plausibly the result of prebiotic chemistry. The analogue computing paradigm describes cells more accurately and reveals them, unmistakably, as the products of a mind.
Article – Viewing cells as integrated multiprocessing analogue computing devices by Royal Truman, Journal of Creation. Vol 40, Issue 3